It’s been called witch’s hair, devil’s hair, devil’s guts, devil’s ringlets, scaldweed, beggarweed, fireweed, strangleweed, strangle tare, hairweed, pull-down, hailweed, and hellbine — the parasitic plant dodder doesn’t get a whole lot of love.1 If you do much hiking in southern California, you’re probably used to seeing huge, yellow-orange masses of dodder draping vegetation. Many people assume it’s invasive, but it’s actually native to California.

Noble Canyon, Pine Valley, CA 07/07/19
Dodder is in the genus Cuscuta, which contains between 100 and 170 species, all of them parasites. It has a world-wide distribution. Cuscuta used to be treated as the only genus in the family Cuscutaceae, but it’s now been incorporated into the morning glory family (Convolvulaceae). The various species can be yellow, orange, or red. At least one species, Cuscuta reflexa or giant dodder, is green. (That one’s found in India, so I probably won’t be posting any photos of it here.)

Cowles Mountain, San Diego County 05/31/19
Cuscuta is classified as a stem parasite, because it invades the stems of other plants (as opposed to their roots). Like all parasitic plants, dodder evolved from photosynthetic ancestors. At least some species still retain traces of chlorophyll, although not nearly enough to survive without a host. Generally, if a plant is parasitic, but still does some of its own photosynthesis, it’s called a hemiparasite. If, on the other hand, it has totally lost the ability to photosynthesize, it’s called a holoparasite. Dodder seems to be an edge case. Some of the articles I’ve read confidently state that it’s a hemiparasite. Others just as confidently call it a holoparasite. To some extent, it probably depends on the species. As mentioned earlier, the Indian species — C. reflexa, is green, so it retains more chlorophyll than the other species and probably photosynthesizes at least slightly. When it comes to the other dodders, the various articles can’t seem to agree on whether they photosynthesize just a little bit or none at all.
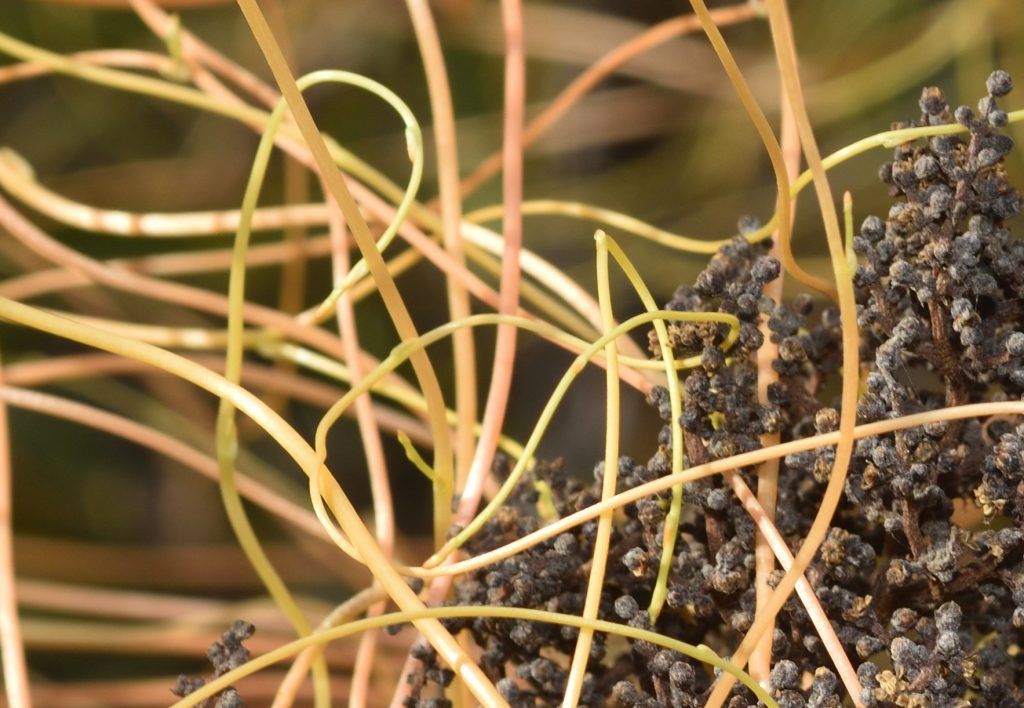
Cowles Mountain, San Diego County 07/23/19
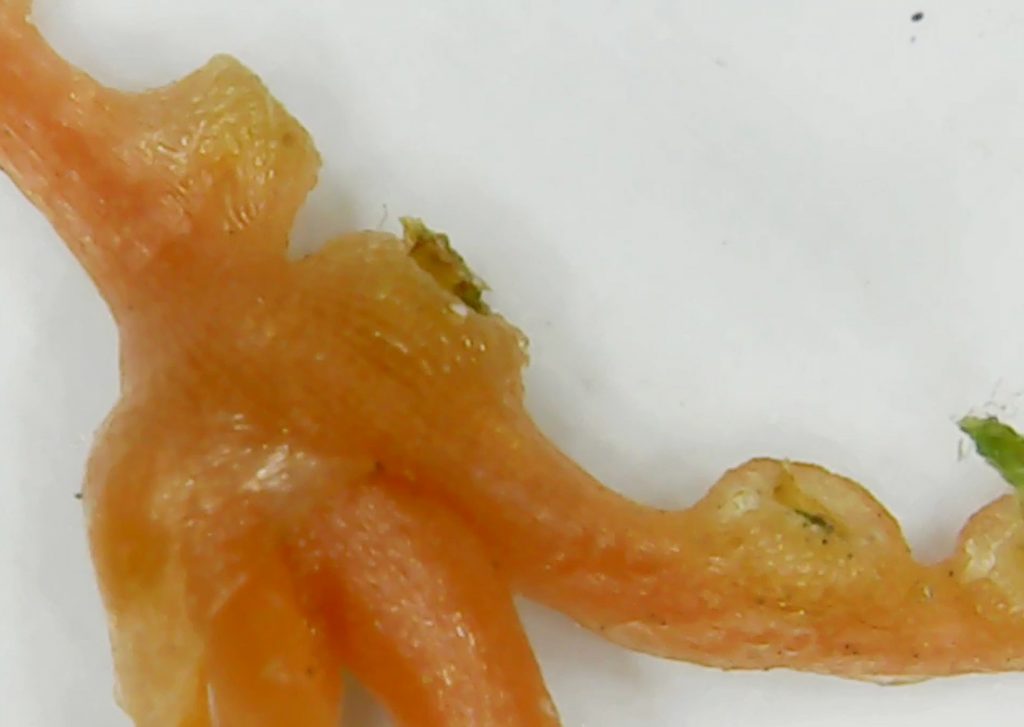
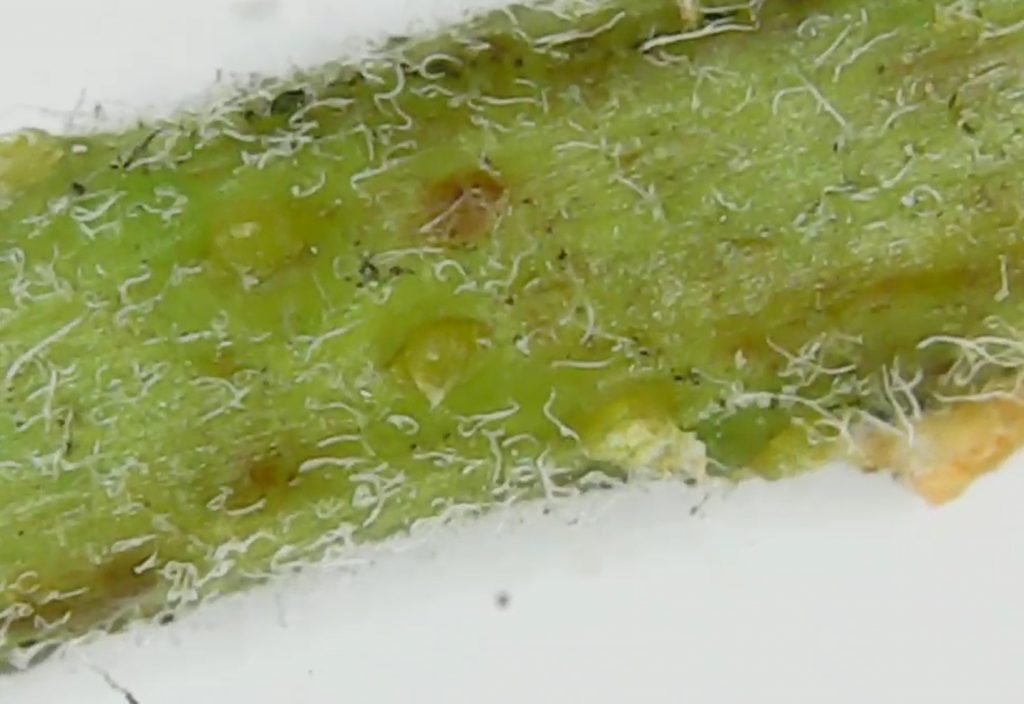
When a dodder stem contacts a plant, it wraps itself around the plant. (It even wraps itself around itself, as you can see from the photos in this post). If the plant is a potential host, the dodder will produce very thin, modified roots called haustoria (singular haustorium), which burrow into the stems of the host plant and invade its vascular system, tapping into both xylem and phloem.2 The dodder then proceeds to extract all the water, sugar, and nutrients it needs from the other plant.
A Closer Look at Haustoria
The following description is based on an article published in the online journal “Frontiers of Plant Science“. You can read that article here.
When a dodder stem comes into contact with an appropriate host, it goes into an “attachment phase”, in which the cells at the contact point develop into a secondary meristem.3 This secondary meristem forms an adhesive disk or “prehaustorium”, which adheres to the stem of the host plant. Cuscuta even induces the host plant to produce sticky substances of its own to reinforce the connection.
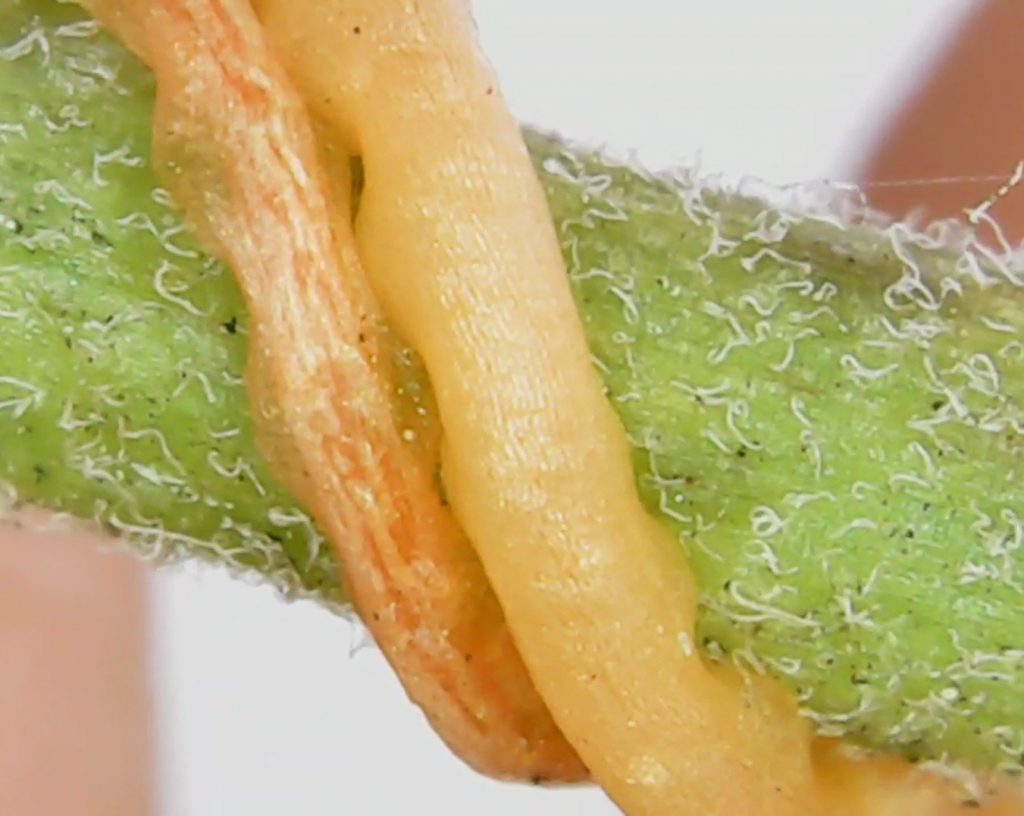
San Diego County 05/31/19
Next comes the “penetration phase”, in which a haustorium grows from the adhesive disk and penetrates the stem of the host. Cuscuta secretes enzymes that work to degrade the cell walls of the host and the developing haustorium forces its way through the weakened or ruptured walls. Meanwhile, the dodder stem continues to grow longer, attaching a second prehaustorium, then a third, and so on.
Cells at the tips of the haustoria form “searching hyphae”, which search for xylem and phloem. When hyphae come into contact with one of the sieve cells of the phloem, they grow around the cell “like the fingers of a hand”. The hyphae then fuse with the cell so completely that it’s hard to tell where the parasitic hyphae end and the host cell begins.

Similarly, when the searching hyphae find xylem tissue, the dodder stimulates the host xylem to develop synchronously with its own xylem tissue (formed within the hyphae), resulting in a continuous tube of xylem connecting the two plants.
To quote from the referenced article:
“The haustorium […] is the defining feature of all parasitic plants, representing the interface where nutrients, solutes, and carbohydrates are exchanged between host and parasite. […] This interface also allows the exchange of macromolecules between the host plant and the parasite.”
And:
“… the impressive extent of exchanged macromolecules such as RNAs confirms the haustorium as an ‘open door’ between host and parasite that seems not especially guarded.”
Cuscuta can reproduce asexually from bits of stem spread by birds or other animals. Dodder is a flowering plant, however, so it can also grow from seed. Most, if not all, species are annuals, so I suppose it has to regrow from seeds each year. A newly germinated seedling has roots, but little or no chlorophyll, so it has to reach a host as soon as possible. The endosperm of the seed, which is much like the yolk of an egg, contains enough food to keep the young plant alive for 5 to 10 days after germination, but if it fails to find a host within that time period, it dies. Experiments have shown that dodder locates potential hosts by sensing airborne chemicals released by the plants. In other words, it smells them. Dodder has been shown to be sensitive to a number of different volatile compounds and to be repelled by others. Once a seedling attaches itself to a host, its roots are no longer needed, so they wither away.
Dodder seeds don’t have any obvious dispersal mechanism — they simply drop to the ground. The plants probably rely on the dispersal of bits of stem by animals to spread to new areas.

Cowles Mountain, San Diego County 05/31/19
Cowles Mountain, San Diego County 07/12/19
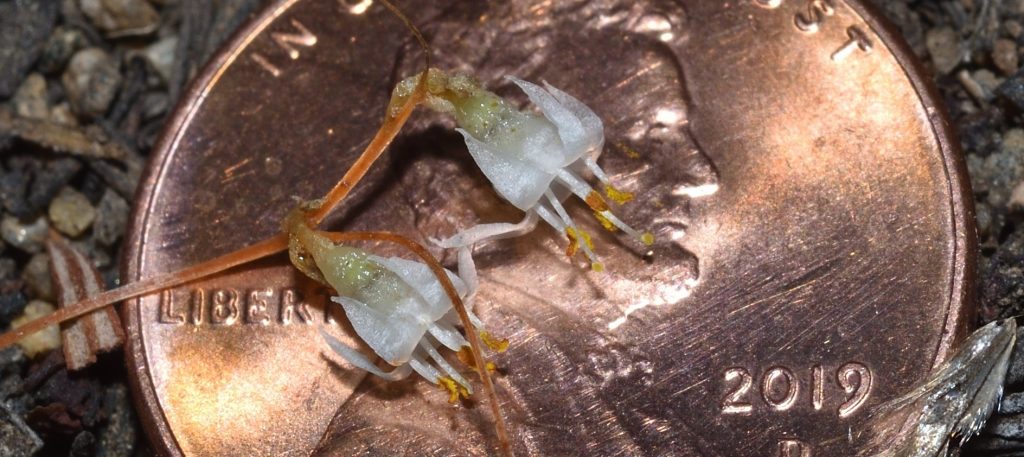
Many people who are familiar with dodder don’t realize that it’s a flowering plant. That’s probably because they’ve never bothered to take a close look. Dodder produces flowers in abundance, but they’re very tiny — around 3 mm wide. In most species, they’re white or cream-colored, so they don’t stand out against the pale yellow-orange of the stems.
There are a number of species of dodder in southern California, but the two most common ones are Chaparral or California dodder (C. californica) and canyon dodder (C. subinclusa). I’ve seen both species growing on Cowles Mountain in Mission Trails Regional Park, just west of San Diego. California dodder grows at or near the bottom of the mountain. It infests mostly buckwheat. The flowers are short, white, and urn-shaped.
The canyon dodder in the park grows mostly on laurel sumac. Its stems are noticeably thicker than those of California dodder. The flowers are also white, but longer and more tube-shaped. The petals are joined for maybe two-thirds of their length.
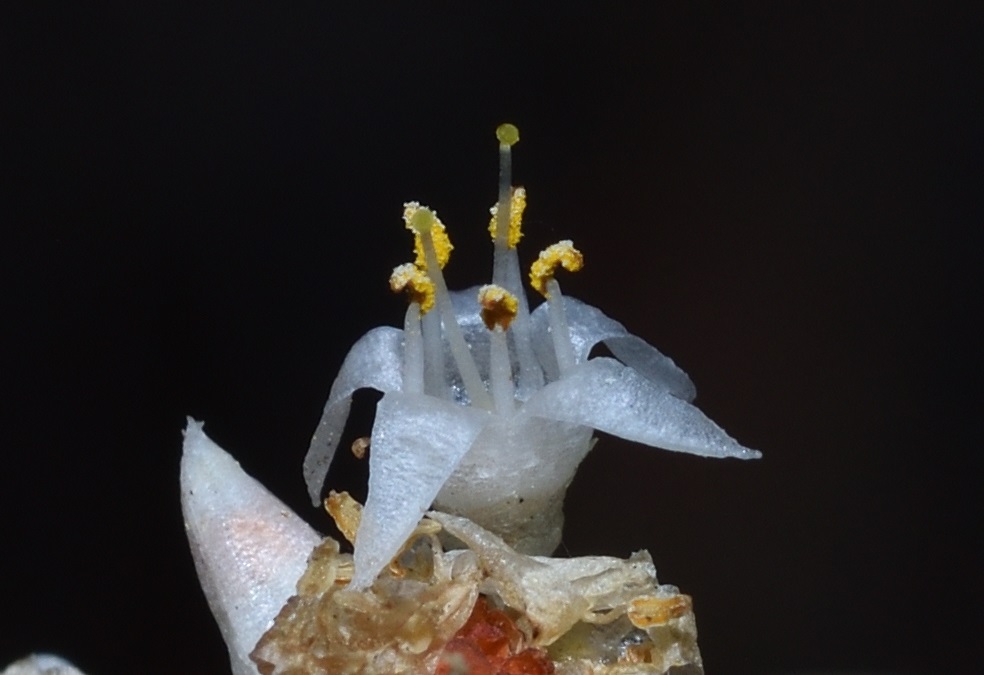
A dodder flower has five petals. The petals are joined together near the base, but peel back at the ends to expose five stamens4 and two pistils.5 The pistil of a dodder consists mostly of a style — a long, thin stalk — sporting a very small, round stigma on the end. When a pollen grain sticks to a style, it grows a thin tube that penetrates the style and follows it down to the ovary, which it fertilizes. As a flower matures, the styles grow longer. They may not grow equally, though. In many species, one style will grow noticeably longer than the other.
Cowles Mountain, San Diego County 07/12/19

The reddish plant matter to the left of the flower is part of the buckwheat host.
Cowles Mountain, San Diego County 07/12/19
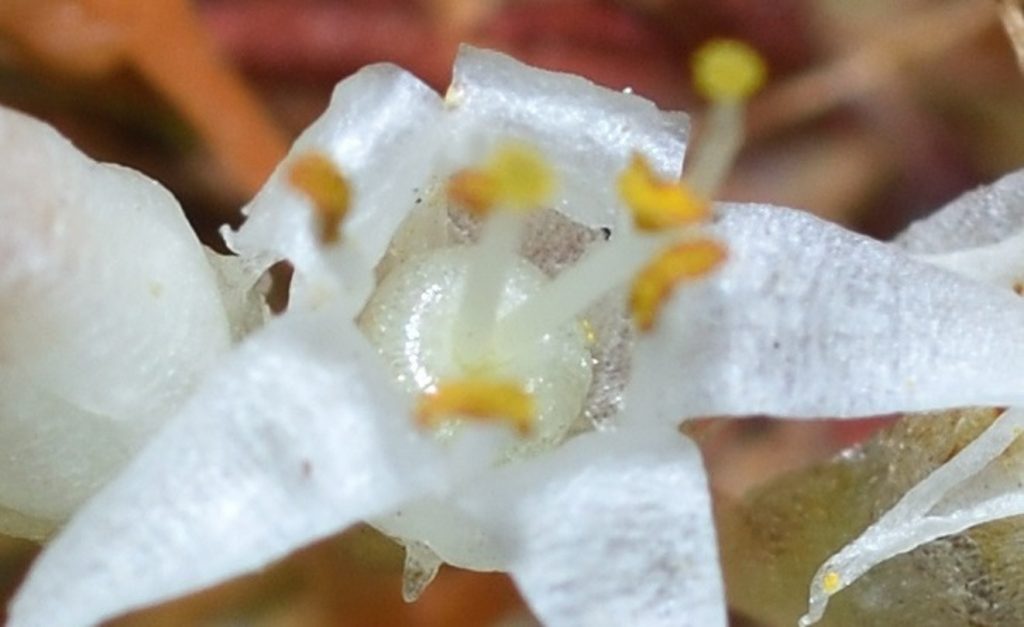
Cowles Mountain, San Diego County 07/12/19
Why would a flower have two unequal styles? This represents two different methods of assuring reproductive success. An insect flying from flower to flower will pick up pollen from one flower and transport it to the next. The long pistil stands a better chance of getting pollen from the visiting insect stuck to it, so it has a better chance of picking up pollen from a different plant. The short pistil, on the other hand, has a better chance of receiving pollen from the stamen growing next to it. In other words, one pistil favors cross-pollination and the other favors self-pollination.
The whole point of sexual reproduction is to give a species a better chance of coping with changes in the environment by producing offspring with many different characteristics. If the environment changes in such a way that one individual has less chance of survival, maybe another individual with different characteristics will stand a better chance. So, all things being equal, cross-pollination is better than self-pollination. On the other hand, what if the pollinators that a flower usually relies on are in short supply? In that case, the plant can still reproduce by self-pollination.
Which is better — cross-pollination or self-pollination — can vary with circumstances. For instance, many plants have evolved to take advantage of disturbed ground. When a large tree falls, clearing a space in the forest, or a fire kills all the vegetation in an area, some plants have evolved to quickly colonize the newly vacated plot of ground, squeezing in a few generations before other plants crowd them out. For this kind of plant, self-pollination may be the more successful strategy, simply because it’s quicker — the plant doesn’t have to wait for a bug to come by or for the wind to blow a few pollen grains of the right sort in its direction. Believe it or not, some flowers have evolved to grow flower buds that never open! They still have stamens and styles, but the pollen from the stamens always ends up on the styles in the same bud.
As a plant species encounters different environments, it will often evolve different pollination strategies that allow it to adapt to those environments. If some members of a species evolve a new strategy that is so different from the old strategy that they are no longer able to breed with the plants that use the old strategy, then those members have formed a new species.
In his Master’s thesis, which you can read online here, Michael Wright discusses the evolution of sexual reproduction in Cuscuta. He comes to the conclusion that the evolution of two styles of unequal length was crucial to the success of the genus. To quote Dr. Wright, “The more flexible floral design enabled Cuscuta to evolve different mechanisms of reproductive assurance in coordination with their exploitation of novel host species and new pollination environments.”
Some of the examples he gives are fascinating. In one subspecies, a style tends to collect pollen from it’s own flower near its tip, but, as it grows longer and the stamens begin to wither and die, the style bends over, so that its lower part is exposed to any visiting insects. In this way, if it collects a pollen grain from an insect, that grain will likely be closer to the bottom of the style than any pollen that it picked up from its own stamens. So the tube that grows from the foreign pollen may be able to reach the ovule first. Thus, preference is given to the potentially more beneficial foreign pollen.
The Consequences of Intimacy
A single Cuscuta plant will routinely infect multiple host plants and multiple Cuscuta plants will routinely infect the same host. And, as already noted, the haustoria of Cuscuta form a very intimate connection with the vascular tissue of the host plant, allowing all sorts of things to pass between them. These several facts have some important consequences:
The transfer of viruses. Viruses seem to pass freely from an infected host plant to Cuscuta and from there to an uninfected host. Sometimes a virus is able to infect the dodder, as well as the host plant. In this situation, the dodder can go on to pass on the virus to other host plants even if all the original hosts have died. In other cases, Cuscuta may be immune to infection by the virus. This does not prevent it from transferring the virus between hosts, however.
Horizontal gene transfer (HGT). HGT is most familiar in microbes. Bacteria, for instance, routinely exchange DNA. This is one reason they are able to evolve resistance to antibiotics so quickly. What scientists have only recently begun to appreciate is that HGT can also occur in plants and animals. The mechanisms are not fully understood and it probably doesn’t happen very often, but there is good evidence that parasitic plants, such as Cuscuta, can exchange genes with their hosts. It’s likely that much of Cuscuta‘s success as a parasite is a result of its ability to incorporate useful genes from host plants and express them in its haustoria.
Communication between hosts. The fact that Cuscuta steals resources from its host plant is obviously detrimental to the host. There’s no getting around that. However, it doesn’t benefit a parasite if its host dies. So, perhaps it’s not so surprising that a parasite will sometimes do things that actually benefit the host. There is experimental evidence that when a dodder connects multiple host plants, it forms a communication network between them, passing useful info from plant to plant. See the section below for more details.
How Dodder Helps Its Hosts
A study published in PNAS6 showed that when two host plants are connected by a Cuscuta bridge and one of the hosts is attacked by an insect, the dodder will pass signals to the other host that cause that host to react in a way that makes it more resistant to attack. (Click here to read the original paper.)

The study was done on Cuscuta australis. The insect pest in the study was tobacco cutworm (Spodoptera litura). Several host plants were used.
A number of experiments were done in the study. In a typical experiment, C. australis was allowed to infect two host plants growing close together, but not in contact. S. litura was allowed to feed on one of the host plants. I’ll call this plant A and I’ll call the other plant (which was not being fed on) plant B. After a period of time (say 48 hours), leaves from both host plants and vines from the dodder were collected and subjected to RNA-sequencing analysis to determine what changes had occurred in gene expression (up-regulation or down-regulation of the genes).
When an insect feeds on a leaf of a plant, the other leaves will typically start to produce chemicals that make them less attractive to the insect. The results of this study showed that the same thing happened in plant B. Apparently, when an insect feeds on a leaf of a host plant, the leaf produces signals that cause its other leaves to ramp up their defenses. These same signals are passed along by the dodder to any other host plants that it is attached to, causing them to follow suit.
The same experiment was done on plants that were close together, but not connected by dodder. In this case, plant B did not ramp up its defenses. This shows that whatever signals were being produced by plant A, they were only passed on to plant B if A and B were connected by dodder. Surprisingly, the results were similar even when plants A and B were in different families.
After collecting the leaves and vines for analysis, S. litura was allowed to feed for a time on plant B. Data was then collected on the amount of damage caused by the insects. This data showed that when a Cuscuta bridge was present, plant B experienced less insect damage, lending support to the conclusions drawn from the RNA-sequencing analysis.
Some Clues About How Dodder Became Dodder
A genetic analysis done on C. australis found that dodder split from its common ancestor with Ipomoea (the largest genus in the morning glory family) around 33 million years ago. This analysis produced a number of other interesting results. Apparently, the common ancestor of Cuscuta and Ipomoea experienced a whole-genome triplication event before the split. This is not too uncommon in plants. Such an event in an animal would almost certainly be fatal, but plants tend to be less affected by such things. In fact, having multiple copies of a gene often allows the extra copies to go on to evolve new functions, thus helping to drive evolution. Chances are, it was this triplication event that led to the split between Cuscuta and Ipomoea.
Two other results of this analysis were that Cuscuta experienced accelerated molecular evolution and large-scale gene loss. Both of these findings are typical of parasitic plants, especially holoparasites. Since a holoparasite has no need to photosynthesize and no need to extract resources from the soil, it can safely rid itself of the genes that control those functions. The parasite also has less need to produce substances to defend itself from infection and predation, since it can often use substances produced by its host plant for that purpose.
As for the accelerated molecular evolution, I haven’t been able to find any explicit explanation for that in my reading. My guess would be that the switch to a parasitic lifestyle introduces novel selective pressures that other plants in an area would not experience.
Click here to read this study.